Offering multiple perspectives from many fields of human inquiry that may move all of us toward a more integrated understanding of who we are as conscious beings.
From Pacific Standard, this is an interesting article on how humans are using DNA -- ours and other species' -- to change the world. One wonders if that is such a good thing considering how little we still know about how DNA functions.
How we’ve co-opted our genetic material to change our world. •
Humans and their ancestors have been using tools for millions of years. We owe our prolific capacity for making tools to our DNA, and now we’ve reached the point were we’ve made DNA itself into a tool. We use DNA as a crucial research tool in the lab, we use it to engineer food crops and biofuel-producing microbes, we use it as a forensic tool and a medical diagnostic, and we use it to access our ancient history. We’ve even put DNA to uses that have nothing to do with biology whatsoever, as a nanomaterial with amazing chemical properties. Our genetic material is turning out to be one of our most useful high-tech tools. It didn’t have to be this way. Before the 20th century, scientists didn’t expect the physical make-up of our genes to be something as simple, elegant, and useful as DNA. Darwin, for example, proposed that our genetic material was basically a chemical soup, made of different kinds of molecules that were secreted by each body part and gathered in the reproductive cells. Like the diffuse nebular gases that self-organize into solar systems, our genetic material was often thought to be a complex mix of ingredients that spontaneously organize themselves to direct the development of a new organism. If this theory were true, the science of genetics—and our society—would now be very different. It would be much more difficult, if not impossible, to do many of the things we do with DNA, such as engineer microbes to make drugs or biofuels, or discover our relationship with Neanderthals. Paternity tests and viruses wouldn’t exist. Perhaps life wouldn’t exist either; in the 1930s and ’40s, physicists convincingly argued that a genetic chemical soup was thermodynamically impossible. By that time, biologists were already well on their way to discovering what genes actually are: segments of giant molecules of DNA. Our genetic material turns out to be surprisingly similar to a text, with genes spelled out in a linear string of chemical letters. The analogy to a text isn’t perfect, but it’s remarkably good and partially explains why DNA is such a useful tool. The ability to represent genes as a text on our computers is a boon to biologists, who now analyze genomes with the same text-parsing algorithms that go into spam filters. One of the most basic tools of a molecular biology lab are enzymes that cut, copy, and paste DNA text; without these, much of the last 40 years of biological research would have been impossible. So would commercial genetic engineering, which, aside from its role in agriculture, is increasingly important for producing drugs and chemicals using processes that are more efficient and less environmentally damaging. Because of DNA’s useful properties, “molecular biology” is not only a scientific discipline, but also a set of essential tools used by biologists of all sorts. By manipulating DNA, scientists tackle questions that have little to do with DNA’s biological role. They modify DNA to test hypotheses or to insert chemical sensors into an experimental organism, and they use DNA as a convenient way to read the outcome of an experiment. In my own work, I use DNA “barcodes,” short, easy-to-read sequences of DNA that tag the process I’m interested in. In paternity testing and forensics DNA is merely an identifier; its molecular function is irrelevant. That DNA is a tool with many different biological applications explains the enormous impact of the recent, dramatic improvements in technologies to read and synthesize DNA—DNA science dominates biology more than ever before. We’ve now extended the uses of DNA beyond biology. DNA is not only life’s hackable source code; it’s a nanomaterial with very useful chemical properties. In particular, DNA is a programmable polymer that reliably folds into very small and fantastically intricate shapes. Engineering shapes from folded DNA is called, appropriately enough, DNA origami. Two key properties of DNA make this molecular origami possible: With its 4-letter chemical alphabet, the number of possible designs is huge. There are over a trillion variations of even a very short, 20-unit long DNA segment. And second, strands of DNA like to stick to each other in predictable ways, typically forming the iconic double helix. Using DNA origami, engineers have built all sorts of miniature DNA widgets: motors, sensors, rulers, stencils, boxes, smiley faces, and “dolphin-shaped structures with flexible tails.” These aren’t just demonstration pieces; DNA origami is key element of nanotechnology. In a paper published this month, researchers from MIT and Harvard’s Wyss Institute for Biologically Inspired Engineering describe how they built DNA “molds” to cast precisely shaped gold and silver nanoparticles. These nanoparticles are used in a variety of technologies, and they are typically etched using beams of electrons. But this process is slow and limited in its resolution. By building small molds out of strands of DNA and filling them with gold or silver particles, the researchers were able to cast nano-spheres, triangles, and cubes. They argue that their strategy “points to a new kind of manufacture framework: DNA-directed, digitally programmable fabrication of inorganic nanostructures and devices”—essentially 3-D printing on a nanometer level. As a tool-using species, we’ve long been making tools out of whatever materials we can get our hands on. We’re lucky that we’ve got the DNA to build tools. We’re also lucky that DNA itself makes such a great tool.
Michael White is a systems biologist at the Department of Genetics and the Center for Genome Sciences and Systems Biology at the Washington University School of Medicine in St. Louis, where he studies how DNA encodes information for gene regulation. He co-founded the online science pub The Finch and Pea. Follow him on Twitter @genologos.
Resilience has become a buzzword in the health and psychology press, a word generally defined as an individual's ability to adapt to stress or adversity in healthy ways. But it is a much more complex issue than that.
The article below employs a relational developmental systems model to understanding how resilience is formed. Most previous research has focused on the behavioral and psychosocial aspects of resilience. Dante Cicchetti, in the article below, adopts a much more comprehensive model.
The
pathway to either psychopathology or resilience is influenced by a
complex matrix of the individual’s level of biological and psychological
organization, current experiences, active choices, the social context,
timing of the adverse event(s) and experiences, and the developmental
history of the individual.
In seeking to understand how resilience occurs, or doesn't occur, Cicchetti looked at maltreated children using a multilevel analysis to make sense of why some children develop resilience and others develop psychopathology.
Full Citation: Cicchetti, D. (2010, Oct). Resilience under conditions of extreme stress: A multilevel perspective. World Psychiatry; 9(3): 145–154.
Resilience
has been conceptualized as a dynamic developmental process encompassing
the attainment of positive adaptation within the context of significant
threat, severe adversity, or trauma. Until the past decade, the
empirical study of resilience predominantly focused on behavioral and
psychosocial correlates of, and contributors to, the phenomenon and did
not examine neurobiological or genetic correlates of and contributors to
resilience. Technological advances in molecular genetics and
neuroimaging, and in measuring other biological aspects of behavior,
have made it more feasible to begin to conduct research on pathways to
resilient functioning from a multilevel perspective. Child maltreatment
constitutes a profound immersion in severe stress that challenges and
frequently impairs development across diverse domains of biological and
psychological functioning. Research on the determinants of resilience in
maltreated children is presented as an illustration of empirical work
that is moving from single-level to multilevel investigations of
competent functioning in the face of adversity and trauma. These include
studies of personality, neural, neuroendocrine, and molecular genetic
contributors to resilient adaptation. Analogous to neural plasticity
that takes place in response to brain injury, it is conjectured that it
may be possible to conceptualize resilience as the ability of
individuals to recover functioning after exposure to extreme stress.
Multilevel randomized control prevention and intervention trials have
substantial potential for facilitating the promotion of resilient
functioning in diverse high-risk populations that have experienced
significant adversity. Determining the multiple levels at which change
is engendered through randomized control trials will provide insight
into the mechanisms of change, the extent to which neural plasticity may
be promoted, and the interrelations between biological and
psychological processes in the development of maladaptation,
psychopathology, and resilience.
* * * *
From
the perspective of developmental psychopathology, maladaptation and
mental disorder are viewed as evolving from progressive liabilities in
the organization of biological and psychological systems, resulting in
the undermining of the individual’s efforts to adapt effectively to
stressful and adverse experiences 1,2.
The dynamic interplay between risk and protective forces is conceived
as influencing the developmental course through the impact it has on the
quality of the organization of biological and psychological systems as
the individual develops 3.
Developmental
psychopathologists stress that there is multifinality in developmental
processes such that the manner in which persons respond to and interact
with vulnerability and protective factors at each level of the ecology
(i.e., culture, community, family, and their transactions) allows for
diversity in developmental outcomes 4,5.
Individuals may begin on the same major developmental trajectory, yet
exhibit very different patterns of maladaptation or adaptation. The
pathway to either psychopathology or resilience is influenced by a
complex matrix of the individual’s level of biological and psychological
organization, current experiences, active choices, the social context,
timing of the adverse event(s) and experiences, and the developmental
history of the individual 5.
Understanding
the dynamic transactions between risk and protective factors plays a
central role in building developmentally informed models of prevention.
Through increasing the relative balance of protective processes over
risk factors, the potential for righting the developmental course,
attaining adaptive developmental pathways, and reducing the emergence of
psychopathology may be achieved 4,6.
Just
as deviations from the average expectable environment potentiate some
individuals toward the development of maladaptation, others demonstrate
adaptation in the face of the same challenges 7,8,9.
Thus, it is equally important to comprehend the mechanisms that promote
adaptation among individuals experiencing significant adversity as it
is to investigate the developmental trajectories toward maladaptation.
Research conducted on biological, as well as psychological, protective
factors is critically important for discovering mechanisms and processes
that contribute to the development of either the recovery of function
or resilient adaptation in the face of significant adversity 10,11,12.
DEFINITION AND HISTORICAL CONTEXT
Resilience
is conceived as a dynamic developmental process encompassing the
attainment of positive adaptation within the context of significant
adversity 8,13,14.
There are two critical conditions that are implicit within this
conceptualization of resilience: a) exposure to significant threat,
severe adversity, or trauma; and b) the achievement of positive
adaptation despite major assaults on the developmental process 8,14.
For
four decades, researchers interested in children who develop well in
the context of significant adversity have endeavored to enhance
understanding of the diverse pathways to psychopathology, to elucidate
the processes that eventuate in normal development, and to inform
preventive interventions and social policies that could improve the
lives of vulnerable children and families 7,15,16,17,18.
Investigations in the area of risk and resilience have led scientists
to rethink their prior assumptions about the causes and course of
psychopathology and have resulted in a reformulation of the deficit
etiological models that characterized earlier viewpoints about the
development of children who have experienced disadvantage and great
adversity 9,19,20.
Studies
conducted on individuals at high risk for psychopathology and on
persons with mental disorders frequently portrayed the developmental
course as deterministic, inevitably resulting in maladaptive and
pathological outcomes. Investigations focusing on genetic and biological
predispositions to psychopathology, assaults on development associated
with inadequate caregiving, and traumatic occurrences within the home –
such as child maltreatment and domestic violence, exposure to community
violence, chronic illness, and catastrophic life events – graphically
convey the multiplicity of risks that can eventuate in disordered
outcomes. As researchers discovered that not all high-risk children
manifested the dire consequences that extant theories of psychopathology
predicted, comprehending the processes through which children at risk
did not develop psychopathology became viewed as important for informing
theories on the development of maladaptation and pathology.
Before
investigations on resilience could be initiated, a significant and
illustrious history of research detailing the precursors to, as well as
the contemporary patterns of, stress resistance had to take place (e.g.,
8,21). In many of these early studies, researchers had discovered
evidence of adaptive behavior; however, the nomenclature for labeling
these results as indicative of resilience had not yet emerged.
The
historical roots of resilience can be traced to early programs of
research on individuals with schizophrenia and on persons exposed to
parental mental illness, extreme stress and poverty, as well as on the
functioning of individuals who experienced traumatic occurrences earlier
in their lives 7,15,22,23.
Early investigations of severely disordered schizophrenic patients were
focused primarily on understanding maladaptive behavior, and the subset
of patients who showed relatively adaptive patterns were considered
atypical and afforded little attention. By the middle of the 20th
century, researchers had discovered that people with schizophrenia with
the least severe courses of illness were characterized by a premorbid
history of a relative competence at work, good social relations,
marriage and the capacity to fulfill responsibility (see 23). In a
parallel fashion, studies of children of mothers with schizophrenia
played a crucial role in the emergence of childhood resilience as a
major theoretical and empirical topic 16,19,24.
Additionally, Werner’s longitudinal study 17,18,
that systematically searched for protective forces that differentiated
children with healthy adaptation profiles from those who were
comparatively less well adjusted, was a groundbreaking investigation.
Evidence that many of these children experiencing great adversity
thrived despite their high-risk status led to increasing empirical
efforts to understand individual variations in response to adversity.
Early empirical efforts were primarily focused on the personal qualities
of “resilient children”, such as autonomy or high self-esteem 25.
As work in the area evolved, however, researchers increasingly
acknowledged that resilience may often derive from factors external to
the child 8.
Subsequent research led to the delineation of these sets of factors
implicated in the development of resilience: (a) attributes of the
children themselves; (b) aspects of their families; and (c)
characteristics of their wider social environments 8,25.
In
recent decades, there has been a shift in the focus of empirical
investigations; rather than searching for protective factors,
researchers are increasingly striving to discover the mechanisms
underlying resilient functioning 8.
This focus on processes as opposed to identifying factors has enabled
scientists to design prevention and intervention strategies that are
developmentally sensitive for promoting resilience in persons
experiencing significant adversity or trauma 26,27,28.
Knowledge of the processes contributing to resilient functioning can
enable prevention and intervention scientists to capitalize on periods
of developmental change and transitions as unique opportunities for
promoting positive adaptation during significant adversity or trauma 27,29.
As S. Luthar asserted, “it is far more prudent to promote the
development of resilient functioning early in the course of development
rather than to implement treatments to repair disorders once they are
already crystallized” 7.
Randomized control trial (RCT) preventive interventions may be
conceptualized as true experiments in altering the course of development
30,
thereby presenting opportunities to test existing developmental
theories as well as to provide insights into the etiology and course of
positive adaptational outcomes in individuals experiencing significant
adversity 8,31.
As
research on resilience has evolved and transformed over the years, it
has become clear that the attainment of positive adaptation in the face
of significant adversity involves a developmental progression; new
vulnerabilities and challenges and/or strengths and opportunities often
emerge with changing circumstances over the life course 8.
Resilience is not something an individual “has” – it is a multiply
determined developmental process that is not fixed or immutable. Hence,
it is important to conduct longitudinal studies of the determinants of
resilient functioning. In this regard, longitudinal studies on
resilience should focus not only on assessing the stability of the
construct over developmental time, but also on the ability of formerly
resilient individuals to “bounce back” or to recover positive
functioning after experiencing difficult periods and achieve their prior
resilient adaptation 32.
Moreover, since resilient adaptation may be achieved at any point in
the life cycle, there is a need for research on the achievement of
positive outcomes at different points in development, including in
adulthood and in later life 8.
A MULTILEVEL PERSPECTIVE ON RESILIENCE
Until
the past decade, the empirical study of resilience predominantly
focused on behavioral and psychosocial correlates of, and contributors
to, the phenomenon and did not examine biological correlates or
contributors 8,10,11.
These studies were undertaken prior to the inception of modern
techniques for examining the molecular genetic, neural, and biological
correlates of human behavior and development.
Evidence
from earlier variable-oriented and person-oriented investigations of
resilience converge on a short list of attributes of child and
environment that turn out to be well-established general correlates of
competent adaptation and psychopathology. Although there were
methodological flaws and limitations in the early studies 14,
more contemporary investigations nonetheless continue to corroborate
the factors associated with resilient functioning: (a) close
relationships with competent and caring adults in the family and
community; (b) self-regulation abilities; (c) positive views of self; (d)
motivation to be effective in the environment (i.e., self-efficacy and
self-determination); and e) friendships and romantic attachments with
prosocial and well-regulated peers 12.
Problem-solving skills, foresight in planning, and a future orientation
(all linked to executive functions), active coping strategies, and the
capacity to confront fears directly, minimizing denial, disengagement,
and avoidant coping have all been associated with resilient functioning 7,12,14.
Moreover, optimism, positive emotionality, perceiving stressful
occurrences in less threatening ways and the ability to reframe adverse
experiences in a positive vein, spirituality, and being able to find
meaning amidst trauma have each been linked to resilience 33.
Undoubtedly,
the relative neglect of biology as relevant to developmental theorizing
on the unfolding of adaptive behavioral outcomes in the face of
adversity was primarily due to the paucity of information that existed
about the structural and functional organization of the brain 34,35,36.
There simply was not enough knowledge about brain development and
function to articulate their role in the genesis and epigenesis of
normal and deviant mental processes, let alone in their contribution to
the development of resilient adaptation 33.
Most
of what is known about the causes, correlates, course, and consequences
of resilient functioning in the face of adversity have been gleaned
from investigations that focused on relatively narrow domains of
variables 7,8.
Yet it is apparent from the questions addressed by developmental
psychopathologists that progress toward a process-level understanding of
resilient adaptation will require the implementation of research
designs and strategies that call for the simultaneous assessment of
multiple domains of variables both within and outside of the developing
person 11.
In
the past decade, a number of scientists have urged researchers to
incorporate neurobiological and molecular genetic assessments into their
investigations of the developmental pathways to resilient functioning 10,11,37.
Technological advances in molecular genetics, neuroimaging,
magnetoencephalography, electroencephalographic (EEG) recording, and
hormonal assay techniques have made it more feasible to conduct research
on the development of resilience from a multilevel perspective 11,12.
In
addition, the advent of modern neuroscience, along with its many
associated subdisciplines, represents an unprecedented opportunity to
augment current conceptual and methodological approaches to the study of
resilience. Regardless, it is critically important to keep in mind that
biological domains do not function independently; rather, more commonly
the functioning of one system influences the functional properties of
one or more other systems, through a developmental cascade of
bidirectionally influenced processes 38.
Given this increasing recognition of the importance of considering many
levels of interdependent processes simultaneously, in order to advance
the understanding of a multifaceted phenomenon such as resilience, it is
incumbent upon resilience researchers to meet the challenge of
simultaneously incorporating multiple levels of analysis both across and
within systems 39.
Biological and psychological domains are both essential to include in
basic research on resilience and in resilience-promoting interventions.
Each level both informs and constrains all other levels of analysis.
Moreover, the influence of levels on one another is almost always
bidirectional.
Because different levels of
analysis constrain other levels, as scientists learn more about multiple
levels of analysis, resilience researchers conducting their work at
each level will need to develop theories that are consistent across all
levels. When disciplines function in isolation, they run the risk of
creating theories that ultimately will be incorrect, because vital
information from other disciplines has either been ignored or is
unknown. Just as is the case in systems neuroscience 40,
it is critical that there be an integrative framework that incorporates
all levels of analysis about complex systems in the development of
resilience 11,36.
Resilience in maltreated children: from single-level to multilevel investigation
Growing
up under conditions of child maltreatment constitutes a profound
immersion in severe stress that challenges and frequently impairs
development across diverse domains of biological and psychological
functioning 41.
The ecological conditions associated with maltreatment represent a
severe deviation from the average expectable environment. Maltreated
children are likely to manifest atypicalities in neurobiological
processes, physiological responsiveness, emotion recognition and emotion
regulation, attachment relationships, self-system development,
representational processes, social information processing, peer
relationships, school functioning, and romantic relationships 41.
Accordingly, maltreated children are likely to develop a profile of
relatively enduring vulnerability factors, placing them at great risk
for future maladaptation and psychopathology.
Nonetheless,
not all individuals who have been abused and neglected succumb to the
extreme adversity in their lives. Investigation of how some maltreated
individuals cope adaptively despite experiencing significant stress and
trauma offers an opportunity to discover processes at multiple levels of
analysis that are likely to be germane to effective coping in the face
of adversity, yet less readily detectable under more normative stress
exposure 42.
Discovering how maltreated children develop and function resiliently
despite experiencing a multitude of stressors offers considerable
promise for elucidating developmental theories of coping and for
prevention and intervention.
In a longitudinal
investigation of the pathways to resilience in maltreated children, we
sought to ascertain if there were different pathways to resilient
functioning in maltreated and non-maltreated children (both from
comparable low socioeconomic backgrounds) and to explore whether there
were differences between these groups in resilience, recovery of
function, or decline in functioning over the 3-year period of the study 32.
Maltreated children demonstrated greater dysfunction than
non-maltreated children on several indicators of resilient functioning
(e.g., competence with peers, behavior problems, school functioning,
relationships with adult caregivers). Moreover, many of these deficits
persisted across 2 or 3 consecutive years of assessment. Furthermore,
across each of the 3 years, maltreated children exhibited a lower level
of resilient functioning than did the non-maltreated children.
Additionally, the continuity of maladaptive functioning displayed by
maltreated children across the course of this longitudinal study was
substantial. Taken together, these findings underscore the deleterious
impact that maltreatment experiences exert on competent functioning and
attest to the non-transient nature of their influence.
In
this study, we also constructed pattern groups based on the three
consecutive yearly assessments of resilient functioning in maltreated
and non-maltreated children. Inspection of these pattern groups revealed
that there was a significantly greater percentage of maltreated
children than non-maltreated children in the low resilient functioning
pattern group (40.6% vs. 20%). Furthermore, a greater percentage of
maltreated (9.8%) than non-maltreated children (1.3%) displayed zero
competence indicators, thereby reflecting an absence of resilient
strivings across the 3 year study period. Garmezy 16,24
consistently emphasized that most children maintain the ability to
display some resilience strivings in the presence of chronic and serious
adversity. The complete absence of resilient strivings in nearly 10% of
the maltreated children is cause for great concern, as self-righting
tendencies are vital characteristics of all living organisms. The
consistent absence of such strivings throughout the duration of the
investigation is quite aberrant and alarming.
We also
examined factors that contributed to the development of resilient
functioning in the groups of disadvantaged maltreated and non-maltreated
children. For the maltreated children, the major predictors of
resilient functioning were the personality characteristics of ego
overcontrol (i.e., the ability to monitor and control impulses and
regulate affect) and ego resiliency (i.e., the degree of relative
flexibility in regulating affect and behavior to meet situational
demands), and positive self-esteem. In contrast, for the non-maltreated
children, positive relationships with their mother and other adult
caregivers and ego resiliency played prominent roles in the prediction
of adaptive functioning. Given the high percentage of insecure and
disorganized attachments in maltreated youngsters 43,
it makes sense that relationship factors would be more vital to the
attainment of resilience in the disadvantaged non-maltreated children.
Personality
characteristics and self-system processes were more important in
achieving resilient adaptation in maltreated children. Specifically, the
self-system variables of self-reliance and self-confidence, in concert
with interpersonal reserve (i.e., ego overcontrol), appear to bode well
for the development of resilient adaptation in maltreated children.
Through adopting a more reserved, controlled, and rational way of
interacting and relating (i.e., resilient overcontrol), maltreated
children who function in a resilient fashion may be more attuned to what
is necessary for successful adaptation in their adverse home
environments. It is conceivable that their more overcontrolled style may
protect them from being targets of continued maltreatment incidents. In
contrast, the more affectively expressive style of resilient
undercontrollers may not be well suited for successful adaptation in
maltreating environments, because such styles may provoke attention and
reaction from others that could result in greater risk for maltreatment 44.
Following
the completion of this longitudinal investigation of the psychosocial
processes underlying resilience in maltreated children, we initiated two
multilevel studies. The ecological-transactional perspective that
undergirds this research inherently takes into account multiple levels
of analysis, and allows for combining biological and psychological
mechanisms within the same framework 3,4.
This perspective does not ascribe ascendancy to any level of analysis
over another, and it encourages loosening of conceptual boundaries
between nature and nurture and biology and psychology 45,46,47.
This theoretical perspective thus provides a ready-made structure for
the integration of a multilevel perspective into resilience.
In
the first multilevel investigation of resilience, emotion regulation,
and hemispheric EEG asymmetry in maltreated and nonmaltreated children
from high-stress low socioeconomic backgrounds, we hypothesized that the
positive emotionality and increased emotion regulatory ability
associated with resilient functioning would be associated with
relatively greater left frontal EEG activity 48.
A large body of literature concerning the meaning and correlates of
hemispheric asymmetries in EEG activity has suggested that this
ubiquitous phenomenon indexes a neural system that has emotion-specific
influences whereby the two hemispheres of the cerebral cortex have been
found to be differentially involved in emotion 48.
Specifically, the left hemisphere is associated with positive
emotions/approach behavior and the right hemisphere is linked with
negative emotions/withdrawal behavior. Emotions, and in particular
positive emotion and good emotion regulatory abilities, have
consistently been associated with resilient adaptation 18,49,50.
Thus, the potential connection of hemispheric EEG asymmetry with
resilience lies in their common linkages with emotion and emotion
regulation.
EEG asymmetry across central cortical
regions distinguished between children with high and low resilient
functioning, such that left hemisphere activity characterized those
maltreated children who were adapting resiliently based on our
competence composite index (e.g., good peer relations, adapting
successfully to school, low levels of depressive symptomatology, low
externalizing and internalizing psychopathology) 51.
Moreover, a behavioral measure of emotion regulation, based on 35 hours
of observation of the children, significantly contributed to the
prediction of resilience in maltreated and non-maltreated children.
The
investigation of a neural-level phenomenon such as hemispheric EEG
asymmetry in the context of resilient adaptation reminds us that there
is certainly no one single characteristic that will be ascendant in the
process of resilience over the course of development. Resilience is a
dynamic, interactive process between multiple levels across time, none
of which holds primary importance at any given moment. However, viewed
across development, the relative importance of various biological and
psychological processes, although inevitably interrelated, may also vary
across development.
In another multilevel
investigation conducted in our laboratory, resilient functioning in
maltreated and non-maltreated low-income children in relation to the
regulation of two stress-responsive adrenal steroid hormones, cortisol
and dehydroepiandrosterone (DHEA), as well as the personality constructs
of ego resiliency and ego control, was examined 52.
The steroid hormones we chose to investigate as potential predictors of
resilience are the two primary adrenocortical products of secretory
activity of the hypothalamic-pituitary-adrenal (HPA) axis. The capacity
of individuals to elevate cortisol levels in response to exposure to
acute trauma is important for survival 2.
DHEA exerts an impact upon a diverse array of biological actions,
including effects on the immune, cardiovascular, endocrine, metabolic,
and central nervous systems 53.
As
in the previous single- and multilevel research on the pathways to
resilient adaptation described above, we utilized a composite measure of
resilience that included multi-method, multi-informant assessments of
competent peer relations, school success, and low levels of
internalizing and externalizing symptomatology. We found that ego
resiliency and ego overcontrol and the adrenal steroid hormones
associated with stress (i.e., cortisol and DHEA) made independent and
non-interactive contributions to resilience. Although operating at
different levels of analysis, behavioral/psychological and biological
factors each made unique contributions to resilience.
Prolonged
stress, as is often the case in child maltreatment, can lead to
allostatic load, characterized by cumulative physiological dysregulation
across multiple biological systems, through a cascade of causes and
sequelae that can change the brain, organ systems, and the neurochemical
balance that undergirds cognition, emotion, mood, personality, and
behavior 54,55.
Allostatic load is thought to occur when the adaptation to stress
necessitates that the responses must be maintained over sustained time
periods. Allostasis and allostatic load can be conceived as embodying a
general biological principle – namely that the systems that help the
body adapt to stress, and serve a protective function in the short term,
also may take part in the development of pathophysiological processes
when overused or managed ineffectively.
We found that
higher morning levels of cortisol were related to lower levels of
resilient strivings for the non-maltreated children. High basal cortisol
may indicate that non-maltreated children are experiencing greater
stress exposure and, consequently, are constrained in their ability to
adapt competently. Within the group of maltreated children, differences
in cortisol regulation were found as a function of the subtype(s) of
maltreatment experienced. Physically abused children with high morning
cortisol had higher resilient functioning than physically abused
children with lower levels of morning cortisol. The positive role of
increased cortisol for physically abused children is divergent from the
more general pattern of higher cortisol being related to lower resilient
functioning as we discovered in the non-maltreated and sexually abused
children in this study.
Prior research on
neuroendocrine regulation has indicated that physically abused children
generally exhibit lower levels of morning cortisol secretion 56.
It may be that the subgroup of physically abused children who were able
to elevate cortisol to cope with the life stressors was demonstrating a
greater striving for resilient adaptation. In contrast, the larger
subgroup of physically abused children with lower levels of morning
cortisol may have developed hypocortisolism over time in response to
chronic stress exposure (i.e., allostatic load) 57.
As a result, for these children there may be a diminished capacity to
mobilize the HPA axis to promote positive adaptation under conditions of
ongoing stress. Additionally, we found that the very low level of
resilience among sexually abused children with high basal cortisol may
be a product of their different traumatic experiences and consequences
of chronic excessive vigilance and preoccupation, with commensurate HPA
axis hyperarousal 52.
Finally,
we also discovered that maltreated children with high resilient
functioning exhibited a unique atypical pattern of a relative DHEA
diurnal increase. Maltreated children who have the capacity to elevate
DHEA over the course of the day may be better equipped to cope with the
demands of high chronic exposure to stress and to adapt competently. In
contrast, the non-maltreated children who functioned resiliently did not
exhibit the pattern of diurnal DHEA increase; instead they displayed
the lowest levels of DHEA across the day.
Gene-environment interaction and the molecular mechanisms that promote resilient functioning in maltreated children
Recent
years have witnessed a renascence of interest in investigating the
interaction between genes and environmental pathogens in the development
of psychopathology and resilience 58,59,60.
From a genetic perspective, resilience can be conceptualized as the
extent to which persons at genetic risk for maladaptation and mental
disorder are not affected 61.
Additionally, there may be genetic contributors to resilient adaptation
that protect some individuals in families where there is a high genetic
loading for developing maladaptation and mental disorder from
succumbing to these deleterious outcomes 58.
Moreover, genes are likely to serve a protective function against
environmental insults for some individuals. Thus, it is apparent that
genetic influences on maladaptation and psychopathology operate in a
probabilistic and not in a deterministic manner.
In
gene-environment interaction (GxE), environmental experiences moderate
genetic effects (or vice versa) on normal, psychopathological, and
resilient developmental outcomes. For example, genetic effects on
functioning outcomes may be observed only under certain environmental
contexts or in conjunction with particular histories of experience;
conversely, experience may only relate to outcomes among persons with
specific genetic characteristics 62.
The
majority of GxE studies have investigated polymorphisms in monoamine
oxidase A (MAOA) and serotonin transporter (5-HTT), two of the primary
genes implicated in the maturation of the early developing brain and in
mood, behavior, and responsiveness to stress 58.
The variability exhibited in children’s responses to the environmental
hazard of child maltreatment suggests that this heterogeneity may be
within the hemisphere of genetic influence 59.
The experience of child maltreatment has proven to be a strong
environmental pathogen that has generated a number of provocative
findings which have contributed to engendering interest in research on
GxE (59,60; for meta-analyses, see 65,66).
Caspi and colleagues 62,63
demonstrated GxE effects in a large sample of adults who had
experienced severe early child maltreatment. Specifically, Caspi et al 58
found that adult males who were maltreated early in development and who
possessed the low activity allelic variant of the MAOA gene evidenced
higher levels of antisocial and aggressive symptomatology than did those
individuals who were maltreated early and who had the high activity
variant of MAOA. The latter group demonstrated lower levels of
antisocial and aggressive symptoms 62 than did maltreated adults with the low activity variant of MAOA. In a subsequent investigation, Caspi et al 63
discovered that adults who experienced severe maltreatment in childhood
and who possessed the short (s/s) variant of the 5-HTT gene exhibited
higher levels of depressive symptoms than did adults who had the long
variant (l/l) of the 5-HTT gene and had been maltreated as children. In
contrast, adults in the latter group had significantly fewer depressive
symptoms than did maltreated adults with the short allele variants 63.
Thus, it is conceivable that the high activity MAOA gene polymorphism
and the long variants of the 5-HTT gene may confer protection against
antisocial disorder and depression to adults who have been severely
maltreated in their childhood.
In our laboratory, we
conducted a multigenic study examining the interaction between
polymorphisms of 5-HTT and MAOA genes in a large sample of maltreated
children in relation to depressive symptomatology 67.
Adolescents from low socioeconomic backgrounds with a history of child
maltreatment or no such history were administered a semi-structured
diagnostic interview for mental disorders; moreover, these adolescents
provided buccal cells for genetic analysis. Heightened depressive
symptoms were found among extensively maltreated youth with low MAOA
activity. Among comparably maltreated youths with high MAOA activity,
self-coping strategies related to lower depressive symptoms. The finding
that self-coping strategies and high MAOA activity were related to
lower depressive symptoms calls to mind results from a number of our
studies on resilience in maltreated children. Specifically,
self-reliance and self-determination were found to be predictors of
resilient functioning in maltreated children 32.
It is conceivable that the maltreated children with positive
self-system characteristics who functioned resiliently also may have
possessed polymorphic variants of genes (such as high MAOA activity)
that served a protective function against maladaptation.
Sexual
abuse and the 5-HTT short/short genotype predicted higher depression,
anxiety, and somatic symptoms. This GxE interaction was further
moderated by MAOA activity level. Specifically, we found that sexually
abused adolescents with one or two copies of the 5-HTT short allele had
significantly reduced levels of internalizing symptoms if they also had
the high activity version of the MAOA gene 67.
We
also have begun to decipher co-actions across multiple levels of
analysis through incorporating genetic and multiple physiological
measures in our multilevel research on pathways to resilience in abused
and neglected children. For example, in a longitudinal investigation
that is currently underway in our laboratory, we are employing a
multiple-levels-of-analysis approach to examining the course of
trauma-related psychopathology in maltreated children, as well as the
multilevel processes that contribute to resilient outcomes. In addition
to genotyping relevant candidate genes, we have incorporated multiple
measures of neurophysiological responses to classes of emotion stimuli,
and hormonal, neurocognitive and behavioral functioning. The field can
no longer afford to continue the artificial distinction among genetics,
neurobiology, and behavior in research on the determinants of
resilience.
Neural plasticity and resilience: some potential linkages
Experience-expectant
and experience-dependent mechanisms of neural plasticity are integral
to the very anatomical structure of cortical tissue and cause the
formation of the brain to be an extended malleable process 65,66,67.
Developmental psychopathologists and neuroscientists can utilize this
knowledge as an avenue for understanding the vulnerability and
protective processes of brain development as contributors to the genesis
and epigenesis of psychopathology and resilience. Moreover, because the
mechanisms of plasticity cause the brain’s anatomical differentiation
to be dependent on stimulation from the environment, it is clear that
the cytoarchitecture of the cerebral cortex is shaped by input from the
social environment. Because the human cortex is only diffusely
structured by the genetic plan, and because its eventual differentiation
is highly reactive to the active coping strategies of the individual in
a particular environment, it is highly likely that both normal,
abnormal, and resilient outcomes of this process would encompass a
diverse range of cortical network anatomies and individual
personalities.
Analogous to neural plasticity that takes place in response to brain injury 68,69,70,71, resilience can be viewed as the ability of an individual to recover after exposure to adversity or trauma 9,32.
According to this view, adversity is thought to exert a damaging effect
on one or more neural substrates, and mechanisms of neural plasticity
bring about recovery in an individual. This might lead to the conclusion
that certain individuals, classified as resilient, may have some
increased innate capacity (i.e., plasticity), above and beyond normative
levels, to recover from environmental insults that impact the brain.
This view of resilience conceives of adversity in the environment as
“bad” for the brain, with recovery as an innate property of the brain
itself. This perspective, however, does not consider the impact of a
positive environment (e.g., presence of social supports), or of the
individual’s active attempts at coping, or of protective/plasticity
genes, on such recovery.
Another conceptualization of
resilience would be one of greater than normative resistance to the
impact of environmental adversity on the brain, such that resilient
individuals may not succumb to the potentially damaging effects that
adversity may have on the brain and other biological systems. This view
of brain-adversity interaction would not strictly be classified as
involving neural plasticity. Thus, for these individuals, the term
recovery of function may not apply, in that they did not “lose” function
at all.
The rapid growth in sophisticated techniques
that permit imaging of the brain directly has resulted in the
availability of a variety of methodologies to developmental
psychopathology researchers; many of these methods could be utilized to
examine neural plasticity, as well as brain structure and function, in
detail. These new tools make it possible to now undertake empirical
investigations of the relation between neural plasticity and resilience,
perhaps enabling an examination of the direct linkage of these two
processes. Questions about how neural plasticity may play a role in the
development and maintenance of resilient functioning could be addressed,
as well as whether the mechanisms of neural plasticity may operate
differently in individuals classified as resilient.
Among
the compelling questions about resilient adaptation that could
potentially be addressed utilizing brain imaging methodologies are: (a)
Is brain structure and function different in maltreated and
non-maltreated children functioning resiliently, matched on experiences
of adversity? (b) Is the brain structure and function of resilient
individuals who have experienced adversity different from normal
children reared in non-adverse environments? (c) Are particular areas of
the brain more likely to be activated in resilient than in non-resilient
functioning during challenging or stressful tasks? (d) What aspects of
brain structure and function differentiate individuals who function
resiliently, despite experiencing early adversity, from those who
function in a non-resilient fashion and who encounter adversity early in
life (i.e., what is the role of early experience?) e) Are there
sensitive periods beyond which the achievement of resilience is
improbable or is resilience possible to achieve across the life span?
and f) Are there changes over time in brain structure and/or functioning
in individuals classified as resilient that may reflect processes of
neural plasticity? The inclusion of neuroimaging techniques to the
existing predominantly psychological approaches to charting the pathways
to resilience, along with the additional biological and molecular
genetic methodologies discussed earlier in this paper, could result in
many exciting discoveries about the complex processes that eventuate in
competent outcomes despite the experience of significant adversity.
Aside
from investigating the proximal relation between resilience and neural
plasticity, there are several neurobiologically mediated processes
(e.g., cognition, neuroendocrine functioning) that have a direct
relation to resilient outcome 14,51.
Although such processes exert an impact on resilient functioning,
neural plasticity may, to some degree, be the common, underlying
mechanism that mediates the relation between such processes and
resilience.
Resilience-promoting interventions: a multilevel perspective
Research
on resilience has substantial potential to guide the development and
implementation of interventions for facilitating the promotion of
resilient functioning in diverse high-risk populations that have
experienced significant adversity 27,72.
Such interventions should target protective and vulnerability forces at
multiple levels of influence – culture, community, family, and the
individual.
Although several of the interventions that
have been implemented have employed a multifaceted approach in order to
ensure sensitivity to the diverse transactions between children and
their environmental contexts, to our knowledge there have been very few
interventions that have included biological assessments as part of the
pre-post evaluation battery. Because one of the primary objectives of
the field of prevention science is to intervene in the course of
development to foster the recovery of function and to promote resilient
adaptation in individuals at high risk for psychopathology 6,
it is now essential to utilize a multiple-levels-of-analysis
perspective ranging from DNA sequences to culture in research
evaluations aimed at assessing the efficacy of RCT interventions whose
goal is to foster the development of resilient adaptation.
There
are at least two reasons for the dearth of attention to biological
processes in the evaluation of preventive interventions with children
and adolescents. This lack of attention may partly originate from a
tradition in developmental psychology of measuring biological processes
as indices of heritable, constitutional individual differences
reflecting the neurobiological bases of temperament 73.
This tradition encourages beliefs that biological processes are either
not malleable or are more refractory to positive change as a result of
experience. Because there are bidirectional relations between different
levels of biological and psychological organization, it is essential to
recognize that experience also influences biology 68,74.
Evidence for neurobiological reorganization in response to alterations
in the environment may be less apparent in normative populations where
there likely is greater stability in supportive milieus; however,
investigations of individuals reared in extreme environmental conditions
should enable us to more clearly isolate the components of these
diverse systems, thereby shedding light on the bidirectional effects of
experience and neurobiology.
Random assignment to
adversity or trauma is not possible, but random assignment to
intervention is. If biological systems recover in response to the
intervention, then this provides support for arguments that the systems
under study are sensitive to environmental input during development.
Furthermore, if randomized interventions alter neurobiological systems
associated with disorders, and it can be shown that they mediate changes
in psychosocial and behavioral functioning, then this fosters a better
understanding of the neurobiological bases of the disorder. Moreover,
preventive interventions may contribute to recovery or repair of
biological sequelae in ways that have only begun to be understood.
Improved comprehension of the neurobiological processes that increase
risk of maladaptive development may also suggest novel targets for
preventive intervention. Thus, it is important for prevention scientists
to investigate the means by which changes in experience and
psychological functioning resulting from preventive interventions may
modify biological processes.
Now that animal studies have demonstrated that experience can exert impacts on the microstructure and biochemistry of the brain 75,
a vital role for continuing neural plasticity throughout epigenesis in
contributing to the recovery from various forms of maladaptation and
mental disorder may be suggested. There is growing evidence in the
animal literature that efficacious interventions modify not only
maladaptive behavior, but also the cellular and physiological correlates
of behavior 76,77.
Successful preventive interventions may alter behavior and physiology
through producing alterations in gene expression that create a new
structural reorganization in the brain 76.
One important goal of preventive intervention research is to identify
periods of development when a specific intervention may be more
efficacious so that the intervention can be targeted to that period. A
goal of preventive intervention work that includes measures of
neurobiological processes is to better identify sensitive periods for
intervention 78.
Determining
the multiple levels at which change is engendered through RCT
prevention trials will provide more insights into the mechanisms of
change, the extent to which neural plasticity may be promoted, and the
interrelations between biological and psychological processes in
maladaptation, psychopathology, and resilience 79.
Moreover, preventive interventions with the most in-depth empirical
support, based on integrative multilevel theories of normality,
psychopathology, and resilience, can be implemented in effectiveness
trials in community or real-world settings to reach the broadest number
of people and prevent, alleviate, and ultimately cure, suffering from
mental disorders 80.
Furthermore, the inclusion of biological assessments in evaluations of
interventions designed to foster resilience will enable scientists to
discover whether the various components of multifaceted interventions
each exert a differential impact on separate brain systems. It is thus
possible to conceptualize successful resilience-promoting interventions
as examples of experience-dependent neural plasticity.
Finally,
although the consensus is that resilience is a dynamic developmental
construct that, theoretically, is possible throughout the life course,
it nonetheless is important to ascertain whether the timing of
resilience-promoting interventions is a crucial variable that merits
consideration. Specifically, it will be extremely important to know
whether resilience-promoting interventions are more effective when
implemented in the early years of life. Likewise, are such interventions
more likely to achieve their goal of promoting resilience if they are
instituted as closely as possible to the identification of the adverse
event(s) or experience? The incorporation of a
multiple-levels-of-analysis perspective will enable scientists to learn
whether, for example, resilience-promoting interventions implemented in
the early years of life are better for brain development and
functioning, even if improvement occurs in individuals who receive
resilience-facilitating interventions later in life or receive their
interventions further removed in time from their adverse event(s) or
traumatic experiences.
CONCLUSIONS
It
is important to note that the call for a multilevel perspective in
resilience research and resilience-promoting interventions − that
includes the criticality of conducting genetic and neurobiological, as
well as behavioral, assessments − does not reduce resilience to biology,
let alone to a single biological variable. The inclusion of a
multilevel perspective on resilience should not hearken scientists and
clinicians back to the time when some espoused the view that they were
“invulnerable” children. The incorporation of a multilevel perspective
into research on resilience still requires adherence to a dynamic,
transactional view that respects the importance of context.
We
are in the midst of a truly exciting period for research on the
pathways to resilient functioning in individuals who have experienced
great adversity and trauma. The advances in genomics, epigenetics, brain
imaging, and hormonal and immunological assay techniques will make
important contributions to propelling increased knowledge about the
developmental processes leading to resilience 11,12.
Such enhanced understanding has great potential for the development and
implementation of novel, perhaps even individualized,
resilience-promoting interventions for high-risk children and adults who
are not functioning well due to experiences of adversity and trauma. In
order to comprehend fully how individuals achieve resilient functioning
in the face of adversity, it is incumbent upon us to investigate it
with a commensurate level of complexity.
Acknowledgements
Work on this article was supported by grants from the National Institute of Mental Health (MH083979) and the Spunk Fund, Inc.
This is from Nautilus, this is an interesting look at the future of super-intelligent humans. I suspect we are not likely to see this in my lifetime (I'm 47), but I have no doubt that as we learn more and more about genetics and intelligence, it is inevitable that we will try to create who cities of the super-smart.
The question is will they be smart enough to realize they were created to be pawns in the battles between oligarchies.
Genetic engineering will one day create the smartest humans who have ever lived.
By Stephen Hsu Illustration by Gemma O’Brien
October 16, 2014
Lev Landau, a Nobelist and one of the fathers of a great school of Soviet physics, had a logarithmic scale for ranking theorists, from 1 to 5. A physicist in the first class had ten times the impact of someone in the second class, and so on. He modestly ranked himself as 2.5 until late in life, when he became a 2. In the first class were Heisenberg, Bohr, and Dirac among a few others. Einstein was a 0.5! My friends in the humanities, or other areas of science like biology, are astonished and disturbed that physicists and mathematicians (substitute the polymathic von Neumann for Einstein) might think in this essentially hierarchical way. Apparently, differences in ability are not manifested so clearly in those fields. But I find Landau’s scheme appropriate: There are many physicists whose contributions I cannot imagine having made. I have even come to believe that Landau’s scale could, in principle, be extended well below Einstein’s 0.5. The genetic study of cognitive ability suggests that there exist today variations in human DNA which, if combined in an ideal fashion, could lead to individuals with intelligence that is qualitatively higher than has ever existed on Earth: Crudely speaking, IQs of order 1,000, if the scale were to continue to have meaning.
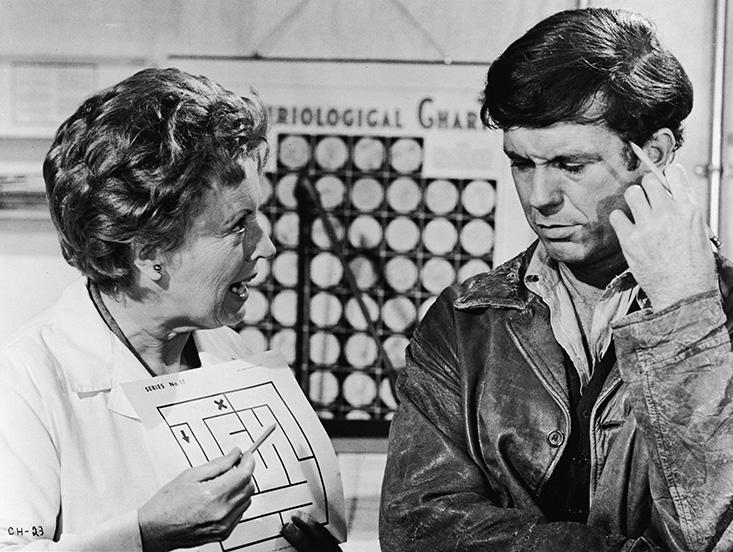
The Overnight Genius: Actor Cliff Robertson, who plays the part of bakery worker-turned-genius Charly (spelled Charlie in the novel), studies an illustration of a maze in this scene from the 1967 film adaptation of Flowers for Algernon.Photo by Cinerama/Courtesy of Getty Images In Daniel Keyes’ novel Flowers for Algernon, a mentally challenged adult called Charlie Gordon receives an experimental treatment to raise his IQ from 60 to somewhere in the neighborhood of 200. He is transformed from a bakery worker who is taken advantage of by his friends, to a genius with an effortless perception of the world’s hidden connections. “I’m living at a peak of clarity and beauty I never knew existed,” Charlie writes. “There is no greater joy than the burst of solution to a problem… This is beauty, love, and truth all rolled into one. This is joy.” The contrast between a super-intelligence and today’s average IQ of 100 would be greater still.
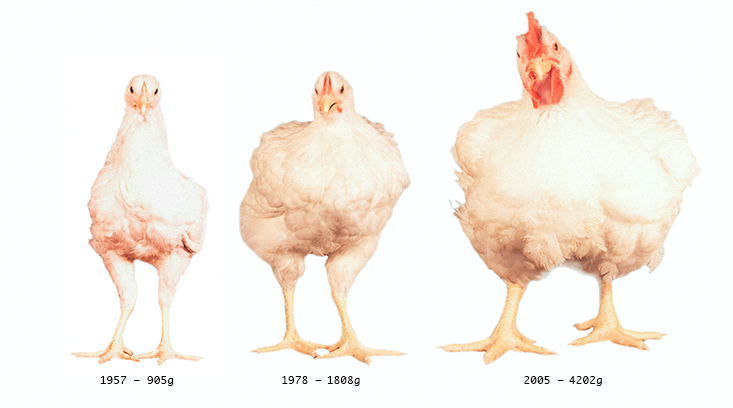
The possibility of super-intelligence follows directly from the genetic basis of intelligence. Characteristics like height and cognitive ability are controlled by thousands of genes, each of small effect. A rough lower bound on the number of common genetic variants affecting each trait can be deduced from the positive or negative effect on the trait (measured in inches of height or IQ points) of already discovered gene variants, called alleles. The Social Science Genome Association Consortium, an international collaboration involving dozens of university labs, has identified a handful of regions of human DNA that affect cognitive ability. They have shown that a handful of single-nucleotide polymorphisms in human DNA are statistically correlated with intelligence, even after correction for multiple testing of 1 million independent DNA regions, in a sample of over 100,000 individuals. If only a small number of genes controlled cognition, then each of the gene variants should have altered IQ by a large chunk—about 15 points of variation between two individuals. But the largest effect size researchers have been able to detect thus far is less than a single point of IQ. Larger effect sizes would have been much easier to detect, but have not been seen. This means that there must be at least thousands of IQ alleles to account for the actual variation seen in the general population. A more sophisticated analysis (with large error bars) yields an estimate of perhaps 10,000 in total.1 Each genetic variant slightly increases or decreases cognitive ability. Because it is determined by many small additive effects, cognitive ability is normally distributed, following the familiar bell-shaped curve, with more people in the middle than in the tails. A person with more than the average number of positive (IQ-increasing) variants will be above average in ability. The number of positive alleles above the population average required to raise the trait value by a standard deviation—that is, 15 points—is proportional to the square root of the number of variants, or about 100. In a nutshell, 100 or so additional positive variants could raise IQ by 15 points. Given that there are many thousands of potential positive variants, the implication is clear: If a human being could be engineered to have the positive version of each causal variant, they might exhibit cognitive ability which is roughly 100 standard deviations above average. This corresponds to more than 1,000 IQ points.
Supersize me: The breeding of domesticated plants and animals has changed some populations by as much as 30 standard deviations. Broiler chickens, for example, have increased in size more than four times since 1957. A similar approach could be applied to human intelligence, leading to IQs greater than 1,000.Zuidhof, M.J., Schneider, B.L., Carney, V.L., Korver, D.R., & Robinson, F.E. Growth, efficiency, and yield of commercial broilers from 1957, 1978, and 2005. Poultry Science 93, 1-13 (2014).
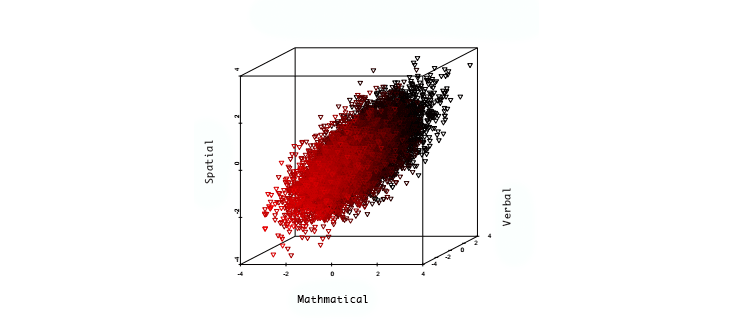
It is not at all clear that IQ scores have any meaning in this range. However, we can be confident that, whatever it means, ability of this kind would far exceed the maximum ability among the approximately 100 billion total individuals who have ever lived. We can imagine savant-like capabilities that, in a maximal type, might be present all at once: nearly perfect recall of images and language; super-fast thinking and calculation; powerful geometric visualization, even in higher dimensions; the ability to execute multiple analyses or trains of thought in parallel at the same time; the list goes on. Charlie Gordon, squared. To achieve this maximal type would require direct editing of the human genome, ensuring the favorable genetic variant at each of 10,000 loci. Optimistically, this might someday be possible with gene editing technologies similar to the recently discovered CRISPR/Cas system that has led to a revolution in genetic engineering in just the past year or two. Harvard genomicist George Church has even suggested that CRISPR will allow the resurrection of mammoths through the selective editing of Asian elephant embryo genomes. Assuming Church is right, we should add super-geniuses to mammoths on the list of wonders to be produced in the new genomic age. SOME of the assumptions behind the prediction of 1,000 IQs are the subject of ongoing debate. In some quarters, the very idea of a quantification of intelligence is contentious. In his autobiographical book Surely You’re Joking, Mr. Feynman!, the Nobel Prize winning physicist Richard Feynman dedicated an entire chapter to his quest to avoid the humanities, called “Always Trying to Escape.” As a student at the Massachusetts Institute of Technology, he says, “I was interested only in science; I was not good at anything else.” The sentiment is a familiar one: Common wisdom sometimes says that people who are good at math are not so good with words, and vice versa. This distinction has affected how we understand genius, suggesting it is an endowment of one particular faculty of the brain, and not a general superlative of the whole brain itself. This in turn makes the idea of apples-to-apples comparisons of intelligence moot, and the very idea of a 1,000 IQ problematic. But psychometric studies, which seek to measure the nature of intelligence, paint a different picture. Millions of observations have shown that essentially all “primitive” cognitive abilities—short and long term memory, the use of language, the use of quantities and numbers, the visualization of geometric relationships, pattern recognition, and so on—are positively correlated. The figure below displays graphically the ability scores of a large group of individuals, in areas such as mathematical, verbal, and spatial performance. The space of the graph is not filled uniformly, but instead the points cluster along an ellipsoidal region with a single long (or principal) axis.
Smart is smart: The Project Talent study looked at the mathematical, verbal, and spatial skills of over 100,000 ninth-graders, as displayed in this scatterplot. Ability in one area was positively correlated with ability in the other two.
These positive correlations between narrow abilities suggest that an individual who is above average in one area (for example, mathematical ability) is more likely to be above average in another (verbal ability). They also suggest a robust and useful method for compressing information concerning cognitive abilities. By projecting the performance of an individual onto the principal axis, we can arrive at a single number measure of cognitive ability results: the general factor g. Well-formulated IQ tests are estimators of g. Does g predict genius? Consider the Study of Mathematically Precocious Youth, a longitudinal study of gifted children identified by testing (using the SAT, which is highly correlated with g) before age 13. All participants were in the top percentile of ability, but the top quintile of that group was at the one in 10,000 level or higher. When surveyed in middle age, it was found that even within this group of gifted individuals, the probability of achievement increased drastically with early test scores. For example, the top quintile group was six times as likely to have been awarded a patent than the lowest quintile. Probability of a STEM doctorate was 18 times larger, and probability of STEM tenure at a top-50 research university was almost eight times larger. It is reasonable to conclude that g represents a meaningful single-number measure of intelligence, allowing for crude but useful apples-to-apples comparisons. Another assumption behind the 1,000-IQ prediction is that cognitive ability is strongly affected by genetics, and that g is heritable. The evidence for this assumption is quite strong. In fact, behavior geneticist and twins researcher Robert Plomin has argued that “the case for substantial genetic influence on g is stronger than for any other human characteristic.”2
In twin and adoption studies, pairwise IQ correlations are roughly proportional to the degree of kinship, defined as the fraction of genes shared between the two individuals. Only small differences due to family environment were found: Biologically unrelated siblings raised in the same family have almost zero correlation in cognitive ability. These results are consistent over large studies conducted in a variety of locations, including different countries. In the absence of deprivation, it would seem that genetic effects determine the upper limit to cognitive ability. However, in studies where subjects have experienced a wider range of environmental conditions, such as poverty, malnutrition, or lack of education, heritability estimates can be much smaller. When environmental conditions are unfavorable, individuals do not achieve their full potential (see The Flynn Effect).
Sidebar: The Flynn Effect
The Flynn effect, named after the philosopher James Flynn, refers to a significant increase in raw cognitive scores over the last 100 years or so—the equivalent of two standard deviations in some cases. This raises a number of thorny issues. Were our ancestors idiots? Is cognitive ability really so malleable under environmental influence (contrary to what has been found in recent twin studies)? The average person 100 years ago was massively deprived by today’s standards— much more so than we would ever be allowed to reproduce in a modern twin study. United States gross domestic product per capita is eight times higher now, and the average number of years people spend in school has increased dramatically. In the America of 1900, adults had an average of about seven years of schooling, a median of 6.5 years, and 25 percent had completed four years or less. Modern twin and adoption studies only include individuals raised in a much smaller range of environments—almost all participants in recent studies have had legally mandated educations, which in the U.S. includes at least several years of high school. There is a revealing analogy with height. While taller parents tend to have taller children (i.e., height is heritable), significant gains in average height which mirror the Flynn effect (amounting to an almost +2 standard deviation change) have been observed as nutrition and diet have improved.
SUPER-INTELLIGENCE may be a distant prospect, but smaller, still-profound developments are likely in the immediate future. Large data sets of human genomes and their corresponding phenotypes (which are the physical and mental characteristics of the individual) will lead to significant progress in our ability to understand the genetic code—in particular, to predict cognitive ability. Detailed calculations suggest that millions of phenotype-genotype pairs will be required to tease out the genetic architecture, using advanced statistical algorithms. However, given the rapidly falling cost of genotyping, this is likely to happen in the next 10 years or so. If existing heritability estimates are any guide, the accuracy of genomic-based prediction of intelligence could be better than about half a population standard deviation (meaning better than plus or minus 10 IQ points). Once predictive models are available, they can be used in reproductive applications, ranging from embryo selection (choosing which IVF zygote to implant) to active genetic editing (for example, using CRISPR techniques). In the former case, parents choosing between 10 or so zygotes could improve the IQ of their child by 15 or more IQ points. This might mean the difference between a child who struggles in school, and one who is able to complete a good college degree. Zygote genotyping from single cell extraction is already technically well developed, so the last remaining capability required for embryo selection is complex phenotype prediction. The cost of these procedures would be less than tuition at many private kindergartens, and of course the consequences will extend over a lifetime and beyond. The corresponding ethical issues are complex and deserve serious attention in what may be a relatively short interval before these capabilities become a reality. Each society will decide for itself where to draw the line on human genetic engineering, but we can expect a diversity of perspectives. Almost certainly, some countries will allow genetic engineering, thereby opening the door for global elites who can afford to travel for access to reproductive technology. As with most technologies, the rich and powerful will be the first beneficiaries. Eventually, though, I believe many countries will not only legalize human genetic engineering, but even make it a (voluntary) part of their national healthcare systems. The alternative would be inequality of a kind never before experienced in human history.
Stephen Hsu is Vice-President for Research and Professor of Theoretical Physics at Michigan State University. He is also a scientific advisor to BGI (formerly, Beijing Genomics Institute) and a founder of its Cognitive Genomics Lab. References 1. Hsu, S.D.H. On the genetic architecture of intelligence and other quantitative traits. Preprint arXiv:1408.3421 (2014). 2. Plomin, R. IQ and human intelligence. The American Journal of Human Genetics65, 1476-1477 (1999).


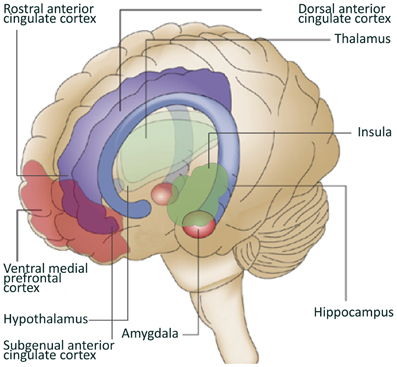
The sentiment is a familiar one: Common wisdom sometimes says that people who are good at math are not so good with words, and vice versa. This distinction has affected how we understand genius, suggesting it is an endowment of one particular faculty of the brain, and not a general superlative of the whole brain itself. This in turn makes the idea of apples-to-apples comparisons of intelligence moot, and the very idea of a 1,000 IQ problematic.